Theme

The thread: Three numbers

An infinite-dimensional spectrum is projected onto three cone responses, and everything colour science can do — and every way it fails — follows from that single collapse.
Four standard illuminants, and how little they have in common. Spectral power distributions for A, D50, D65, E, on one scale. Illuminant A rises steeply toward the red; the daylight illuminants carry the atmosphere's absorption structure; E is flat by definition. All four are ordinarily called white. What light is

A spectrum is not a colour

What arrives at the eye is a function of wavelength. What the eye reports is three numbers. Keeping the two apart is the single most useful habit in the subject, and almost every confusion in applied colour comes from letting them merge.

A spectrum, weighted three ways, and the three numbers left over. The illuminant D65 above; below, the same spectrum multiplied by each matching function. The area under each product is one coordinate of XYZ. Everything else about the spectrum — its shape, its structure, all its remaining degrees of freedom — is discarded here. What the eye does

Three numbers

A spectrum has as many degrees of freedom as anyone cares to give it. The eye reports three. Everything colour science can do, and every way it fails, follows from that one collapse.
Two different spectra that are the same colour. Two reflectance curves differing by 92 per cent RMS, and the two patches they produce under D65: identical to ΔE00 = 6.2e-14, which is arithmetic noise rather than a small number. Both patches are inside the sRGB gamut, so neither has been clipped into agreement. What the eye does

Two spectra, one colour

Metamerism is usually described and almost never demonstrated. It does not have to be — the metameric black space is enormous, so a matching pair can be constructed to order, verified, and then made to come apart by changing the light.

The CIE 1931 colour-matching functions. The three functions that turn a spectrum into three numbers. They are all positive, which is why XYZ exists — the RGB functions they were derived from are not. ȳ is by construction the luminous efficiency function, which is why luminance comes out of Y. What the eye does

Why colour is exactly three-dimensional

Matching every wavelength with three primaries requires, for some wavelengths, a negative amount of one of them. That physical awkwardness is why the colour-matching functions were transformed into XYZ, and why the horseshoe is curved.

triphosphor fluorescent — three narrow phosphors plus the mercury lines, and the white it produces. The spectral power distribution of a triphosphor source, normalised to its own peak, and the colour a perfect white reflector takes under it: chromaticity (0.3379, 0.3389), correlated colour temperature 5258 K at Duv -0.0035. The white looks ordinary. The spectrum producing it does not. What light is

A lamp is not a blackbody

A fluorescent tube puts a third of its light into four mercury lines. A white LED is a blue spike with a hole beside it. Both are sold by a colour temperature, and a colour temperature says nothing about either.
The same two surfaces, weighed by each system. A long-wavelength and a short-wavelength surface under D65, with their relative luminance under the photopic curve and under the scotopic one. Under daylight vision the red surface is 1.33 times the blue; under rod vision it is 0.15 times, a reversal by a factor of 9.0. The swatches are the photopic appearance, which is the only one a display can produce: rod vision has no colour, and drawing a guess at it would be an invention. What the eye does

The eye that has no colour

Rods outnumber cones twenty to one, work alone below a hundredth of a candela, and are absent from the centre of gaze. Between dusk and a lit room both systems run at once, and neither standard curve describes what is happening.

How far a match comes apart when the observer changes. A broad source and a three-primary source, solved at each primary width so the pair is an exact tristimulus match for the CIE 1931 observer. The pair is then handed to the 1964 observer, and the gap between them is plotted. For the observer they were built for the gap is arithmetic noise at every width. For the other it grows as the primaries narrow, reaching 0.012 at 10 nm — and displays have been getting narrower for twenty years. Where the model breaks

Whose eyes

The standard observer is an average over seventeen people, and no reader is it. What that costs was small when displays were broad and grows every time the primaries get narrower.
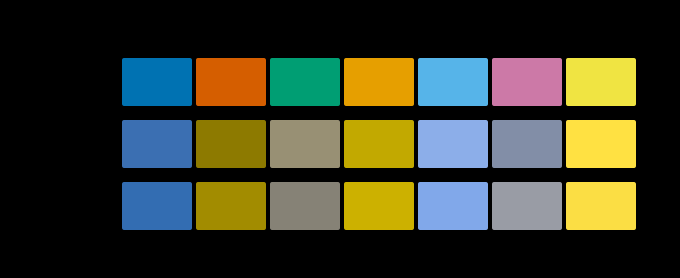
One palette under normal vision and two dichromacies. The same 7 colours simulated by the Brettel–Viénot–Mollon construction at severity 1.0. protanopia and deuteranopia collapse the red-green distinctions. This shows which discriminations survive, not what anybody sees. What the eye does

Three cones, two axes

The retina does not send three receptor signals down the optic nerve. It sends a sum and two differences, and the reason falls out of the statistics of natural light rather than out of anything the eye intended.

Three lightness scales, seventy years apart. Munsell value, CIELAB's L* and CIECAM16's J against luminance, all rescaled to run 0 to 100. Each is somebody's answer to how evenly spaced lightness steps map onto light. They put the midpoint of the scale at 19.8%, 18.4% and 28.0% of the white's luminance respectively — close enough to be three measurements of one thing, far enough apart to be three measurements rather than one restated twice. Matching and measuring

Colour by catalogue

A colour order system arranges physical samples on a regular lattice so a person can find one and name it. The space it samples is not regular, and everything interesting about such systems is what happens at that mismatch.
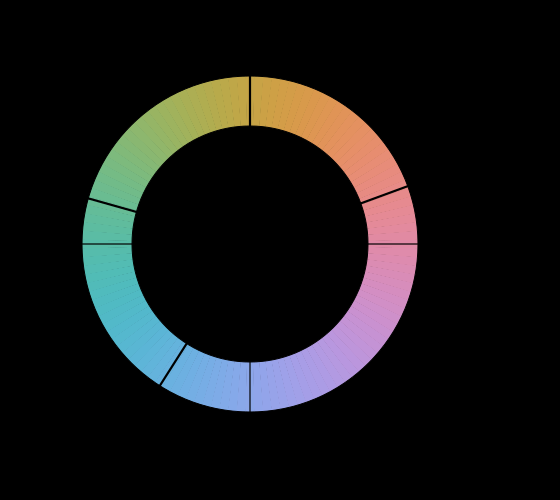
The four unique hues, and the axes they are said to define. A constant-lightness, constant-chroma ring in CIECAM16, with the four unique hue anchors marked and CIELAB's a and b axes drawn through the same circle. If a* really were the red-green axis the anchors would fall on the crosshairs. Unique red sits 25° off, and the four are not 90° apart in any case. Hatched sectors are hues this display cannot reach at this chroma. What the brain does

Why there are four unique hues

Observers agree that four hues are elementary and that no colour is reddish green. Nothing in the three receptors predicts either fact, and the axes of every standard colour space miss the four by tens of degrees.

How far three channels drift from eighty-one, per bounce. One room, one geometry, one reduction to three channels, and the only thing changing is how many bounces of the Neumann series are kept. At one bounce the two agree to 2.5e-13 — the only reflectance in that path is the floor's, which is flat, and a flat reflectance is one of the few three numbers carry exactly. Every bounce after it multiplies another non-flat reflectance into the spectrum, and three numbers cannot carry a product they were never given the factors of. The curve levels off at ΔE00 = 2.38 because the light has run out, not because the disagreement has. What a scene does

Rendering in three numbers

Almost every renderer ever shipped bounces red, green and blue rather than a spectrum. The error that costs is exactly zero at the first product and grows at every one after it — because three numbers cannot carry a product they were never given the factors of, and each bounce is another product.

Why blue and yellow make green. 7 mixtures between a blue and a yellow pigment, mixed in Kubelka–Munk — K/S summed by concentration and inverted back to reflectance — and plotted against the straight line joining the two endpoints. The path bows towards green by 0.099 in chromaticity, and the reason is in the spectra rather than in the eye: the blue reflects below about 520 nm and the yellow above about 500, so the only band both return is the overlap between them. Mixing lights adds spectra and lands on the chord; mixing pigments intersects them and does not. What a scene does

Why blue and yellow make green

The oldest fact in colour, and the usual explanations are wrong. It is not because green sits between blue and yellow, and it is not a fact about the eye at all — it is that the only band both pigments return is their overlap, and the overlap of a blue and a yellow reflectance is green. Computed, the mixing path bows away from the straight line by a measurable amount.

What no surface can be more colourful than. The MacAdam limits at 4 lightnesses under D65, each computed by sweeping two-transition reflectances over the whole band and keeping those that land at the target luminance factor. This is a physical bound rather than a gamut: a reflectance above 1 is a surface that emits, so no pigment anybody invents will ever put an object colour outside these curves. The boundary shrinks steeply as the surface lightens, from 0.310 at Y = 0.1 to 0.028 at Y = 0.9 — a very light surface has almost no room to be colourful, and that is physics rather than pigment chemistry. Drawn against it is sRGB at the same luminance factor rather than as a primary triangle, because a triangle is what a display can reach at some luminance and the bound is what a surface can reach at one; matched properly, sRGB covers 36% at Y = 0.1, 40% at Y = 0.3, 40% at Y = 0.6, 21% at Y = 0.9. The faint triangle is the familiar figure, kept only to show how much it misleads. What a scene does

No surface can be that colourful

There is a hard bound on object colour that no pigment will ever move, and it follows from a reflectance being at most 1. Its boundary is generated by two numbers, it shrinks by a factor of eleven from dark to light — and measured against it properly, sRGB reaches 40% of what a surface could be at mid lightness while Rec. 2020 reaches 106%.
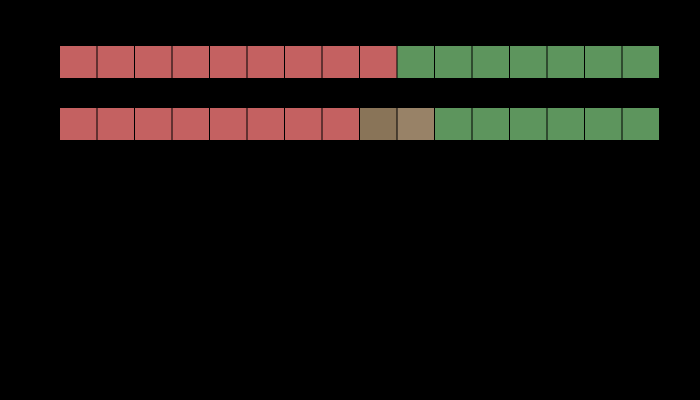
An edge at 4:2:2, and the colour it arrives as. Above, the row as it was sent and as it arrives after the two chroma planes are averaged 2 samples at a time. Below, the colour difference at each sample. The worst is ΔE00 = 25.88, at a luma step of 0.058 across the edge — an edge of nearly equal luminance. Nothing is wrong with the codec: it discards the differences the eye resolves worst, and this edge is made of nothing else. What it takes to deliver it

Colour thrown away on purpose

Every video format in use discards three quarters of its colour information and keeps all of its luminance, because the eye resolves fine colour detail badly. On an edge that carries luminance the loss is exactly zero. On an edge of nearly equal luminance it is a colour difference of forty-three, and the two edges are the same edge to the codec.

Contrast sensitivity, three channels, normalised to each channel's peak. Spatial frequency in cycles per degree against relative sensitivity. The luminance channel runs to 50 cycles per degree, red–green to 12 and blue–yellow to 8, each by the same criterion of 5 per cent of that channel's own peak. Only the luminance channel dips at low frequency; the two chromatic ones are low-pass, so a chromatic edge of any size at all is seen at its full contrast. What the eye does

How fine a colour edge can be

The eye resolves a lightness pattern to about fifty cycles per degree and a red–green one to twelve. Every colour difference here is quoted as though a patch had no size, and the same difference is plainly visible at one scale and gone at another.

The L cone's sensitivity at three axial pigment densities. Each curve is normalised to its own peak, so the only difference visible is shape. Raising the density from 0.1 to 0.9 widens the curve from 113.6 to 145.9 nm at half height while the peak stays within 5 nm of where it was. That is Beer–Lambert saturating: at the peak the pigment already absorbs nearly everything, so more of it can only catch more light in the wings. What the eye does

A cone absorbs its own light

A photopigment's absorbance is a property of a molecule; a cone's sensitivity is that molecule stacked in a column deep enough to absorb most of what arrives. The stacking broadens the curve by thirty-five nanometres, and two observers differing in nothing else disagree about a match that is exact for one of them.

Photons caught by one cone in one integration time, under D65. Each curve is one cone class, counting isomerisations during a 0.1 s integration through a pupil that closes as the light rises. At 1000 cd/m² a long-wavelength cone catches about 11522 and at 0.001 it catches 0.12 — which is where the square root of the count stops being a small correction and starts being the signal. The rate works out at 30 isomerisations per second per troland, inside the published band of 5–50. What the eye does

Colour goes first in the dark

A cone reports a count, and a count carries the square root of itself as noise. Counting the photons says where colour vision stops — a chromatic difference runs out four hundred times sooner than a lightness difference of the same size — and says just as clearly that in daylight the eye is nowhere near that limit.

Cone density, out from the centre of gaze. Quoted landmarks with logarithmic interpolation between them: 199,000 cones per square millimetre at the fovea, 9,500 at ten degrees — a factor of 21. The shaded bands are the two standard observers' fields. The 2° observer averages over a region whose density falls by 3.3× between its centre and its edge and the 10° observer by 12.4×, which is what "a 10° field" contains and is why the two sets of matching functions are different shapes rather than the same shape scaled. What the eye does

Colour stops at the edge of sight

Cone density falls twenty-one-fold between the centre of gaze and ten degrees out, and the three channels give out at three different rates — so a colour difference in the periphery does not merely shrink, it turns. At the exact point of fixation there are no short-wavelength cones at all.

Grassmann's four laws, exact — and the two things that break them. For a linear observer every one of the four is exact and the residual is floating point, which is the control that makes the two failures below measurements rather than artefacts. Rods break a cone-metameric match by 23 per cent of a rod excitation at dusk; bleaching breaks it by 0.59 per cent of a cone excitation in the sun. Both are stated as fractions of a receptor's own response, so they can be put on one scale. Matching and measuring

The laws that make colour add up

Colorimetry is an integral, and an integral assumes matching is linear. Grassmann's four laws are exact for a linear observer, to floating point — and they fail at both ends of the light range, by two different mechanisms, leaving colorimetry an operating band of three and a bit decades that no standard states.

One match, and what it says about the observer making it. The anomaloscope: a monochromatic 589 nm yellow set against a mixture of 545 and 670 nm. Only two cone classes respond at those wavelengths, so the match is two equations in two unknowns and has one solution for any observer whose two pigments differ. The bar is the fraction of the accepted band; the mark is the solution. A normal observer accepts 0.7 per cent of the scale; an observer whose two pigments are the same accepts all of it, because their two equations are one equation twice. Nothing here is fitted to clinical data: the pigments are the same template used for every observer here, at stated peaks, and the match is the solution of the linear system. Matching and measuring

One match names the observer

A yellow at 589 nanometres set against a mixture of 545 and 670 is two equations in two unknowns. It has one solution for a normal observer, a solution somewhere else for an anomalous one, and no unique solution at all for a dichromat — whose two equations are one equation twice.
One light, two eyes. The same stimulus through two sets of ocular media differing only in macular pigment (0.35 and 0.41) and lens age (55 and 55 years). Compared under one white the two differ by ΔE00 1.00; compared with each eye adapted to its own long-run white — which is what the visual system does — by 0.00. The second number is why nobody notices, and the first is why a person who has had one lens replaced reports that the other eye has turned yellow. Where the model breaks

Nobody here has two eyes

One person's two eyes differ in macular pigment and lens density, so the same light produces two colours — a whole ΔE00 apart for an ordinary pair, seven for one replaced lens. Adaptation hides it exactly, which is why nobody notices and why nothing in colorimetry has a term for it.

A fourth primary, swept — every setting an exact match, none of them the same. Four primaries matching three numbers leave one degree of freedom. Along the horizontal axis it is the fourth primary's share of the white's luminance; at each value the other three powers are solved exactly, so every point on this plot is a floating-point-exact match for the reference member — worst residual 1.3e-15 — and no colorimeter can tell them apart. What the population sees runs from 13.7 ΔE00 at the ninety-fifth percentile to 17.3, a factor of 1.26. The best setting is the largest share the arithmetic admits, so what stops it is not colour but the requirement that four powers stay positive. Matching and measuring

Four primaries have a choice

Three primaries matching three numbers have one answer. Four have a family of them, every member exact to floating point for the observer they were solved for — and the members are not equally good for anybody else, so a display with a fourth primary has a setting that is robust to who is looking at it and a setting that is not.

The drift window, asked about each channel in turn. Every spatial frequency a channel can resolve, drifting at v degrees a second, arrives at f × v hertz; the bar is the range of v over which all of them stay above a quarter of that channel's temporal peak. The luminance band is closed at both ends — 0.018 to 0.71 degrees a second — because its temporal sensitivity has a dip at zero to fall into. The chromatic bands have no slow edge at all, because chromatic temporal sensitivity is low-pass: a stationary chromatic pattern sits at the top of its own sensitivity. The mark is the measured drift, and it is inside all three. What the eye does

The drift is a luminance mechanism

The eye's own drift was shown to sit inside a band of speeds that keeps every spatial frequency modulating, and the band was quoted as though it were about vision. Asked about colour, it has no slow edge at all — a stationary chromatic pattern needs no eye movement whatever. And a stabilised chromatic pattern is the first thing to fade.

Coming back from a bleach, against the clock already measured. A 94 per cent bleach, and the pigment returning at its own time constant of 120 seconds. The lower curve is the site's slow neural adaptation constant, 60 seconds, started from the same place — it is finished while the chemistry is barely half done. Regeneration does not speed up because the light went away: the rate constant is the same one it always was, which is why the recovery is slow while the bleaching was fast. What the eye does

The slowest clock is chemical

An earlier essay here joined the afterimage to the adaptation clock and named what was still missing — a third gain, upstream of both, in the pigment itself. It is twice as slow as anything measured before it, it leaves a coloured after-tint from a white field, and at steady state it cancels exactly, which is why nobody has ever needed to model it.

207 essays on this thread, page 1 of 9 · all threads · all essays